See more of our articles in your search results.
You’ve typed the same password forty times, and one morning your fingers just do it while your mind is somewhere else entirely. Or you’ve driven the same route to work so often that you arrive with no memory of the turns. Nobody sat you down and installed that skill. Something in your brain quietly rearranged itself because certain neurons kept talking to each other, again and again, until the conversation got easier.
That something has a name, and it’s older than most of neuroscience. Hebb’s law, more precisely Hebb’s postulate, is the idea that connections between neurons strengthen when one cell repeatedly takes part in making another cell fire. A Canadian psychologist proposed it in 1949, long before anyone could record from a single synapse, and it has turned out to be astonishingly useful and, as I’ll argue, widely misquoted.
Most textbooks reduce it to a rhyme. The rhyme loses a lot.
The real story involves rabbits, cultured neurons, a sea snail, and an uneasy truce between learning and stability.
This article explains Hebb’s law as the neuropsychological basis of learning: what it says, what evidence supports it, where it falls short, and what it means for practice, memory, and recovery.
How many of these have you been "meaning to read" for months?
- 1
 CrosswayDust to DustAging Wisely in an Anti-Aging WorldListen Free On Audible
- 2
 THOUGHT CATALOGThe Mountain Is YouTransforming Self-Sabotage Into Self-MasteryListen Free On Audible
- 3
 Thomas NelsonBreath as PrayerCalm Your Anxiety, Focus Your Mind, and Renew Your Soul (80+ Breath Prayers and Devotional Medita...Listen Free On Audible
What is Hebb’s law, and why is it called a postulate?
Hebb’s law says that when one neuron repeatedly helps to fire another, the connection between them becomes more efficient. It’s the leading proposed explanation for how experience changes the brain, and it’s the conceptual root of what neuroscientists now call synaptic plasticity. Strictly, it’s a postulate, an educated proposal, not a proven law.
Donald Hebb’s own wording described a cell A that is near enough to excite cell B and repeatedly or persistently takes part in firing it. Some growth process or metabolic change, he suggested, then occurs in one or both cells, so that A’s efficiency as one of the cells firing B increases. Notice the phrase “takes part in firing.” That detail matters, and we’ll come back to it.
The famous shorthand, “cells that fire together wire together,” isn’t Hebb’s. Neurobiologist Carla J. Shatz coined it in the early 1990s while explaining how activity sculpts connections in the developing visual system, and it appeared in her 1992 Scientific American article for general readers. Later commentators, including Christian Keysers and David Perrett, have pointed out that the slogan blurs an important feature of Hebb’s actual statement: Hebb stressed a causal relationship (A helps drive B), not mere simultaneity.
That distinction isn’t pedantic. If two neurons fire at the same instant because a third neuron drives them both, there’s no reason for their direct connection to strengthen. Hebb’s version implies sequence and contribution.
Think of it this way. Two coworkers who happen to arrive at the same moment don’t form a working relationship. Two coworkers where one repeatedly prompts the other into action, and the project succeeds, develop a smoother way of working. The first is coincidence; the second is Hebbian.
So the law, in modern terms, has a few ingredients:
- Repetition or persistence: a single co-activation usually isn’t enough.
- Causal contribution: the presynaptic cell must help drive the postsynaptic one.
- Synapse specificity: only the active connections change.
- Lasting change: the efficiency increases for a meaningful period.
Why does a 1949 idea still matter? Because every major modern account of learning, from classical conditioning to artificial neural networks, uses some version of it. And because it connects two fields that rarely shared a vocabulary: psychology, which studies behavior, and physiology, which studies cells.
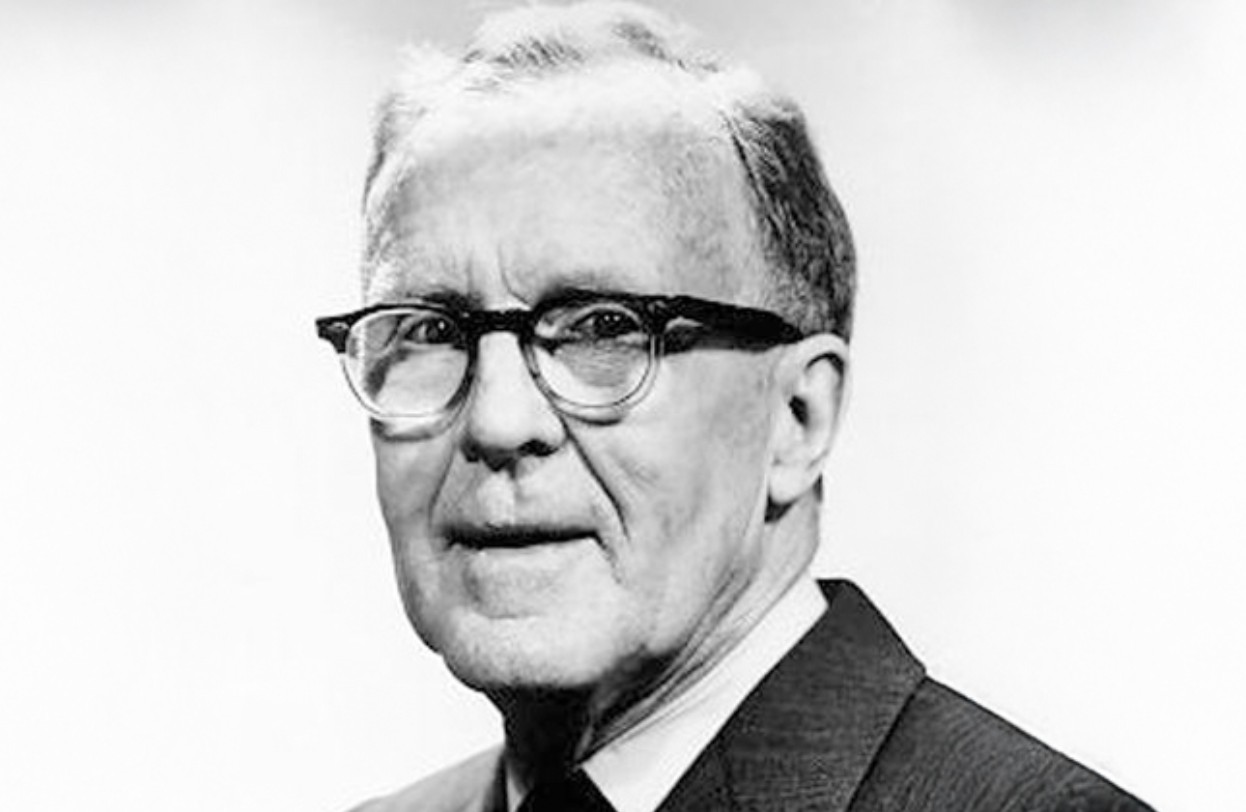
Who was Donald Hebb, and what did he argue in 1949?
Hebb was a psychologist who wanted to bridge the gap between the mind and the brain. In The Organization of Behavior (1949), Donald O. Hebb proposed that learning, memory, and thought could be explained by changes in how neurons connect, and that those changes reflect the history of their activity.
Context helps. In the 1940s, psychology was dominated by behaviorism, which treated the brain as a black box and focused only on stimuli and responses. Neurophysiology, meanwhile, described neurons without much interest in thought. Hebb argued that both fields were missing the connective tissue, and that a theory of mind needed to be built from the activity of cells.
His book introduced three linked ideas. The first was the Hebb synapse, the postulate we’ve just described. The second was the cell assembly, a group of neurons that become interconnected through repeated co-activation so that activating part of the group tends to activate the whole. The third was the phase sequence, a succession of assemblies firing in order, which Hebb proposed as a basis for thought, imagination, and the flow of ideas.
It’s hard to overstate how daring this was. Hebb had no way to observe synapses changing. Techniques that later made long-term potentiation visible would take another quarter century to arrive. He was building a theory of learning from logic, clinical observation, and a few suggestive experiments, including work on how early visual experience shaped later perception in animals.
Hebb also anticipated limits. He recognized that learning in infancy builds the initial assemblies slowly, while adult learning can rely on existing assemblies and proceed faster. That’s an early version of what we now call experience-dependent development.
Consider how that maps to an adult learning a language. A child’s brain builds basic sound categories from scratch through thousands of repetitions. An adult can piggyback on structures built earlier, but also has to overcome the entrenched assemblies of the first language. Same principle, different starting conditions.
Some historians note that Hebb wasn’t entirely original; others had proposed that synapses strengthen with use, and Hebb himself described the idea as an old one. His contribution was to state the principle clearly, tie it to neural architecture, and use it to build an ambitious psychological theory.
Not bad for a man who never saw a synapse change.
What is a cell assembly, and how does it become a memory?
A cell assembly is a group of neurons that, through repeated joint activity, become so strongly interconnected that activating a few of them can ignite the whole set. In Hebb’s theory, an assembly is the neural counterpart of a concept, a percept, or a memory: the physical trace of “this thing.”
Picture the smell of your grandmother’s kitchen. Sensory neurons for the aroma of cinnamon, the visual cortex’s memory of a particular tablecloth, the sound of a kettle, and emotional circuits for warmth all fire together across many visits. Over time, links among them strengthen, and now a whiff of cinnamon alone can reactivate the entire network. You’re not “retrieving a file.” You’re re-igniting an assembly.
Hebb proposed that assemblies could sustain activity for a short while after the stimulus disappeared, through reverberating loops of excitation. Such reverberation might hold information briefly while more durable structural changes take place, a bridge between short-term and long-term memory. Whether this is exactly how short-term memory works remains debated, though reverberating activity in networks is a real phenomenon, and persistent firing has been recorded in prefrontal cortex during working-memory tasks.
The phase sequence extends the idea. Assemblies that frequently fire in succession become linked, so one triggers the next, much as a familiar melody unfolds note by note. That, for Hebb, was a mechanism for chains of thought, planning, and association.
A few properties make assemblies attractive as a model of memory:
- Pattern completion: part of a cue can retrieve the whole memory, as a fragment of a song brings back the rest.
- Graceful degradation: losing some neurons weakens a memory without erasing it.
- Association: assemblies that overlap or co-occur become linked, which fits how memories cluster.
- Distributed storage: a memory isn’t kept in one cell, which fits evidence that damage rarely wipes out a single memory cleanly.
Modern work has substantiated parts of this picture. Researchers have identified groups of neurons in animals, sometimes called engram cells, whose reactivation can trigger remembered behavior. The term “engram,” meaning the physical trace of a memory, predates Hebb, but his assembly concept offered a plausible structure for it.
Still, the details are contested. Nobody has directly observed a human cell assembly encoding a specific memory, and the mapping from assemblies to complex concepts is a hypothesis built partly on inference. The principle is sound; the specifics are evolving.
What’s striking is how well a purely theoretical proposal predicted the architecture of later artificial neural networks, many of which use Hebb-like updates.
What did Bliss and Lømo actually show with long-term potentiation?
They showed that brief, intense activity can strengthen a synapse for a long time. In 1973, Timothy Bliss and Terje Lømo reported that high-frequency stimulation of the perforant path in the hippocampus of anesthetized rabbits produced a sustained increase in the response of dentate gyrus granule cells. The effect later became known as long-term potentiation (LTP).
That was the first direct experimental evidence of a lasting, activity-dependent increase in synaptic strength, and researchers immediately recognized its resemblance to Hebb’s postulate. Follow-up work by Bliss and Gardner-Medwin in unanesthetized rabbits found potentiation that lasted for days, which strengthened the case that LTP could underlie memory, not just short-lived effects of anesthesia.
Why the hippocampus? Because patients with hippocampal damage, most famously the patient known as H.M., lose the ability to form new declarative memories. LTP in hippocampal circuits looked like a plausible cellular mechanism for that kind of learning.
Over the next decades, researchers found several “Hebbian” properties of LTP:
- Cooperativity: multiple inputs active together can push a neuron over threshold for change.
- Associativity: a weak input paired with a strong one can be potentiated alongside it.
- Input specificity: only the stimulated synapses strengthen, not all connections on the cell.
- Persistence: the effect can last hours, days, or longer.
- Dependence on postsynaptic activity: depolarization of the receiving neuron is required.
Associativity is especially elegant. It’s a cellular analog of Pavlov’s dog: a weak signal (bell) gets strengthened if it reliably coincides with a strong one (food). That linkage between a cell-level phenomenon and a classic psychological one helped cement LTP’s reputation as a memory mechanism.
But a note of scientific caution. The tie between LTP and real memory is strong but circumstantial. Blocking LTP often impairs learning in animals, and learning often produces LTP-like changes, yet showing that LTP is the memory mechanism is a harder claim. Some reviewers describe the evidence as compelling but not complete, and the relationship between lab-induced LTP and natural learning is still being refined.
Also, the stimulation used by Bliss and Lømo, a rapid train of electrical pulses, is far more intense than anything a neuron receives in ordinary life. Later work with more natural patterns has shown similar effects, but the original protocol is a blunt instrument.
Blunt or not, it opened a field.
How do NMDA receptors detect “firing together”?
The NMDA receptor, a type of glutamate receptor, works as a molecular coincidence detector. It opens its channel only when two conditions are met at the same time: the presynaptic neuron has released glutamate, and the postsynaptic neuron is already depolarized enough to expel a magnesium ion blocking the channel. That is Hebb’s logic in protein form.
By the 1980s, researchers had worked out a consensus picture: LTP develops when synaptic activity coincides with strong postsynaptic depolarization, which allows the NMDA receptor to open and calcium to flood into the postsynaptic cell. Calcium acts as a trigger for a cascade of events that strengthen the synapse.
Walking through the sequence helps:
- The presynaptic neuron fires and releases glutamate.
- Glutamate binds AMPA receptors, producing a small depolarization in the receiving cell.
- If many inputs arrive together, depolarization becomes strong enough to expel magnesium from NMDA channels.
- With the block removed and glutamate bound, calcium enters through the NMDA receptor.
- Calcium activates enzymes that insert more AMPA receptors into the synapse and, with sustained activity, trigger structural change and gene expression.
The result: the synapse now responds more strongly to the same input. The cell has, in a sense, recorded that this input was part of a successful firing event.
Two things deserve emphasis. First, the NMDA receptor performs a neat logical operation, a molecular “AND gate,” requiring both presynaptic release and postsynaptic depolarization. That is a physical realization of Hebb’s requirement for joint activity. Second, calcium’s role explains why the same mechanism can produce both strengthening and weakening, since different amounts and timings of calcium can recruit different enzymes.
That’s why drugs affecting NMDA receptors have such striking effects on learning and cognition. Blocking them impairs LTP and many forms of learning in animals, while excessive activation can damage neurons through excitotoxicity. Ketamine, an NMDA receptor blocker, has dissociative effects and has also been studied for treatment-resistant depression, though how it works is still under investigation and it should only be used under medical supervision.
Not every form of plasticity depends on NMDA receptors. Some LTP in other pathways, such as mossy fiber synapses, uses different mechanisms, which is a reminder that “the” Hebbian mechanism is really a family of mechanisms.
Still, as a model of how a cell can detect coincidence, the NMDA receptor is hard to beat.
Does the timing between neurons matter?
Yes, a great deal. Blunt claim: simultaneity isn’t enough. Experiments in the late 1990s showed that the order of firing, down to a few milliseconds, determines whether a synapse strengthens or weakens. This phenomenon is called spike-timing-dependent plasticity (STDP).
In 1998, Guo-qiang Bi and Mu-ming Poo reported experiments in cultured hippocampal neurons in which they paired presynaptic input with postsynaptic spikes at precisely controlled intervals. When the presynaptic input came shortly before the postsynaptic spike, the synapse was potentiated. When it came shortly after, the synapse was depressed. The critical window was on the order of tens of milliseconds. Related work by Markram and Sakmann’s group in cortical slices had shown a similar pattern.
This fits Hebb better than a simple coincidence rule. “A helps fire B” implies that A fires first. If B fires first and A arrives afterward, A clearly didn’t contribute to B’s firing, so there’s no reason to strengthen the link, and the synapse actually weakens, a process called long-term depression (LTD).
The STDP rule gives neural circuits a way to encode causality and prediction. Inputs that reliably predict a neuron’s firing get stronger, and inputs that follow it get weaker. That’s useful for learning sequences, and it fits the idea that brains are prediction machines. Many computational models now use STDP to learn temporal patterns.
| Process | What happens | Typical trigger |
|---|---|---|
| Long-term potentiation (LTP) | Synapse strengthens | Strong or repeated coincident activity |
| Long-term depression (LTD) | Synapse weakens | Weak or poorly timed activity |
| STDP, pre before post | Strengthening | Input precedes postsynaptic spike by milliseconds |
| STDP, post before pre | Weakening | Input follows postsynaptic spike |
| Homeostatic scaling | All synapses on a cell scale up or down | Prolonged high or low overall activity |
A caveat about STDP: the neat timing curves come mostly from cultures and slices under controlled conditions. In living brains, neurons receive thousands of inputs, fire in bursts, and are modulated by chemicals such as dopamine and acetylcholine. Real-world plasticity depends on timing, rate, location on the dendrite, and neuromodulation, so the clean curves are a simplification.
Still, STDP refined Hebb’s idea into something testable and rich: not “fire together” but “fire in the right order.”
What would the right order mean for you? Possibly that the sequence of what you practice matters as much as the amount.
What stops Hebbian learning from running out of control?
Imagine a classroom where every student who speaks gets louder applause, so they speak more, and get louder applause, until the room is a roar. That’s the runaway feedback problem with pure Hebbian rules: strengthening makes a connection more likely to fire the cell, which strengthens it further. Left alone, networks would saturate or silence themselves.
Neuroscientist Gina Turrigiano and colleagues helped establish the counterweight, called homeostatic plasticity. In a 2004 review with Sacha Nelson in Nature Reviews Neuroscience, Turrigiano noted that Hebbian mechanisms tend to destabilize circuit activity, so neurons also need processes that keep their average firing within a workable range.
The best-known homeostatic mechanism is synaptic scaling. When a neuron’s overall activity stays too high, it scales down the strength of all its synapses by a common factor. When activity stays too low, it scales them up. Because the scaling is multiplicative, the relative differences between synapses, the pattern laid down by Hebbian learning, are preserved.
That division of labor is elegant. Hebbian plasticity is fast, input-specific, and stores information. Homeostatic plasticity is slow, global, and keeps the system stable. One writes; the other keeps the page from overflowing.
There are other stabilizing tricks too: theoretical models such as the Bienenstock-Cooper-Munro (BCM) rule propose a sliding threshold, so that the amount of activity needed for strengthening shifts up when a neuron has been highly active and down when it’s been quiet. Inhibitory interneurons also play a part, balancing excitation across circuits.
Failures of stability may matter clinically. Researchers have hypothesized that disrupted homeostatic regulation contributes to conditions involving hyperexcitability, such as epilepsy, and perhaps to some features of neurodevelopmental conditions, though the evidence is still developing and the links are far from settled. Treat such claims as promising hypotheses.
The lesson for the Hebb story is that learning in real brains isn’t pure Hebb. It’s Hebb plus a set of safeguards. A theory of memory that ignored stability would predict a brain that crashes.
Notice what that implies about sleep, too. Some researchers propose that sleep helps renormalize synapses after a day of learning, though this is a hypothesis and is debated. It’s one reason sleep deprivation and learning don’t mix.
And it’s a fair reminder: strong theories get better by acquiring caveats.
Did Eric Kandel find Hebbian learning in a sea snail?
Partly. Eric R. Kandel, who won the 2000 Nobel Prize in Physiology or Medicine, studied the giant marine snail Aplysia, whose simple nervous system let researchers trace learning to specific synapses. His work showed that simple forms of learning change synaptic strength, and that long-term memory requires gene expression and the growth of new synaptic connections.
Aplysia’s gill-withdrawal reflex can be modified by experience. A mild touch causes withdrawal; after a shock to the tail, the reflex gets stronger (sensitization), and in a different protocol the animal can learn to associate a touch with a shock (classical conditioning). Kandel’s group traced these changes to the connection between sensory and motor neurons.
The details differ from classical Hebbian LTP in important ways. Much of Aplysia sensitization depends on a neuromodulator, serotonin, acting on the presynaptic neuron, a form of heterosynaptic facilitation, rather than on coincident pre- and postsynaptic firing alone. At the same time, work in this system showed that activity-dependent presynaptic facilitation and Hebbian LTP both contribute to classical conditioning, and that the two interact.
The deeper contribution was molecular. In his 2001 review in Science, Kandel described how repeated training, such as spaced pulses of serotonin, recruits cAMP, protein kinase A, and the transcription factor CREB, which activates genes needed to build new synaptic connections. A single pulse produces short-term facilitation lasting minutes; repeated spaced pulses produce long-term facilitation lasting days and structural growth.
That finding has a practical echo. Spaced repetition produces more durable memory than massed repetition, in sea snails and in students.
Here’s how it connects to Hebb. Hebb proposed that “some growth process or metabolic change” strengthens the synapse. Kandel’s lab supplied a detailed picture of what that growth process looks like: gene transcription, protein synthesis, and new synaptic contacts. In a sense, Aplysia gave Hebb’s vague “growth process” a molecular address.
The caveat: Aplysia is an invertebrate with a few thousand large neurons, and extrapolating to human cognition requires care. Similar molecular pathways, including CREB, are involved in memory in fruit flies, mice, and other animals, which suggests deep conservation, but human memory is vastly more complex.
So Kandel didn’t merely confirm Hebb. He expanded the story from “synapses strengthen” to “here is how, and here’s why practice has to be spaced.”
What does Hebbian learning say about social learning and mirror neurons?
It offers a plausible way to explain why watching someone act can engage your own motor system. Mirror neurons are cells that fire both when you perform an action and when you see someone else perform a similar action. Keysers and Perrett argued in 2004 that such neurons may arise through ordinary Hebbian learning, instead of being innate special-purpose machinery.
The reasoning is simple. When you reach for a cup, you see your own hand, feel the movement, and perhaps hear sounds. Visual and motor neurons repeatedly fire together, strengthening links between the sight of the action and the motor command. Later, seeing someone else do a similar action activates the visual representation, which in turn activates the linked motor representation. A mirror property emerges from correlated experience.
Christian Keysers, a neuroscientist who studies empathy and social cognition, developed this line of thought with David Perrett in a paper titled “Demystifying social cognition: A Hebbian perspective.” Their proposal is that associative learning of this kind could underlie imitation, action understanding, and perhaps aspects of empathy, since seeing someone in pain or disgust can partly reactivate your own related states.
Consider a baby watching her father clap. She has also clapped, felt it, and heard it. Over repeated experiences, the sight of clapping becomes tied to her own clapping circuits. Later, watching someone else clap automatically recruits some of the same neural machinery.
The idea has implications across social learning:
- Imitation becomes easier when the observed action is already in your motor repertoire.
- Emotion contagion might reflect shared representations built through experience.
- Skill learning by observation works best when you can map what you see onto what you can do.
There’s an ongoing debate here. Some researchers argue that mirror neurons are innately specified, others that they’re built by associative learning, and still others that their role in understanding actions and minds has been overstated in popular accounts. The Hebbian account is a serious hypothesis supported by modeling and some developmental data, not a settled fact.
It’s worth noticing how general the idea is. If correlated experience can build cross-modal links between sight and movement, then much of what we think of as “built-in” social ability may be partly learned through the same mechanism as skill learning. That’s a hopeful message for anyone trying to improve social understanding through practice.
And it’s a reminder that Hebb’s law isn’t only about cells in a dish. It’s a hypothesis about how a lifetime of correlated experience becomes a mind.
What does Hebb’s law mean for how you learn and recover?
It suggests that learning is physical work done by repetition, attention, and sequence, and that you can arrange your habits to make it easier. Be careful with the leap from synapses to study tips, since the research on cells doesn’t prove that any given technique works. But several well-tested learning findings are at least consistent with Hebbian principles.
Take Alina (an illustrative composite), learning the piano at 42. She practices ninety minutes on Saturday, nothing the rest of the week, and every Sunday it feels like starting over. Her teacher suggests twenty minutes a day instead. Within a month, passages that once felt alien begin to run on autopilot. Spaced, repeated practice, with sleep in between, usually beats cramming, both in the lab and at the piano bench.
Practical implications that fit the Hebbian picture:
- Repeat, with spacing. Repetition strengthens connections, and spacing across days appears to produce more durable memory, as Kandel’s Aplysia work suggested for a simple system.
- Practice the right thing. Neurons strengthen what they’re actually doing. Practicing errors reinforces errors, so slow, accurate practice often beats fast, sloppy repetition.
- Pay attention. Attention and neuromodulators such as dopamine and acetylcholine influence plasticity, so distracted practice tends to be less effective.
- Mind the sequence. Because timing matters, practice skills in the order you’ll need them, with meaningful context.
- Sleep. Memory consolidation appears to depend on sleep, which supports stabilizing and integrating what you learned.
- Avoid rehearsing what you want to unlearn. Ruminating on a fear or craving can reinforce the circuits you’d like to weaken.
The last point matters clinically. Hebbian-style mechanisms are thought to contribute to the persistence of phobias, habits, and addictive cue responses: repeated pairing of a cue with a reaction strengthens the link. Therapies such as exposure therapy work, in part, by creating new learning that competes with the old association, since the cue now occurs without the feared outcome. It’s a simplified story, since extinction learning is more complicated than erasing a synapse, but the logic holds.
Rehabilitation draws on similar ideas. After stroke, repeated, task-specific practice is a cornerstone of recovery, with approaches such as constraint-induced movement therapy encouraging use of the affected limb. The brain’s capacity for use-dependent reorganization is a reason therapists emphasize repetition and early, intensive practice, although what works varies by patient and condition, and a rehabilitation team can tailor it.
And a note for the skeptic: “neuroplasticity” gets oversold in wellness marketing. Brain-training apps, for example, often improve the trained task without transferring broadly. Hebb’s law explains how learning happens at the synapse; it doesn’t promise that any activity will make you smarter.
The practical rule is straightforward. Whatever you want to be good at, do it, accurately, often, and with attention. Your synapses will do the rest.
FAQs about Hebb’s Law and Learning
What is Hebb’s law in simple terms?
It says that when one neuron repeatedly helps to make another neuron fire, the connection between them gets stronger. Over time, the first cell becomes more effective at triggering the second. Psychologist Donald Hebb proposed this in 1949 as a way to explain learning and memory in terms of brain cells. It’s usually summarized as “cells that fire together wire together,” a phrase popularized by Carla Shatz, not Hebb himself. The simple version leaves out the idea that the first cell has to contribute to the second cell’s firing, which is why scientists emphasize timing and causality in addition to simultaneity.
Did Hebb actually say “cells that fire together wire together”?
No. The phrase was coined by neurobiologist Carla Shatz, who used it in lectures and in a 1992 Scientific American article about how neural activity shapes connections in the developing visual system. Hebb’s own wording, in his 1949 book, described a cell A that repeatedly or persistently takes part in firing a cell B, producing some growth process or metabolic change that increases A’s efficiency. Commentators such as Christian Keysers and David Perrett have noted that the slogan drops the causal element of Hebb’s statement. It’s a handy mnemonic, but a loose paraphrase.
Is Hebb’s law proven?
Mostly supported, not proven in every detail. Experiments on long-term potentiation, beginning with Bliss and Lømo in 1973, show that synapses strengthen after coordinated activity, and NMDA receptors provide a plausible molecular mechanism. Spike-timing-dependent plasticity experiments refined the idea. But connecting those cellular effects to specific memories in living brains remains hard, and other mechanisms, including homeostatic plasticity and neuromodulation, also shape learning. Most neuroscientists treat Hebbian plasticity as a core principle that needs supplementing rather than a complete theory. It’s a very successful framework with known limits, which is how most useful scientific ideas end up.
What is the difference between Hebbian learning and long-term potentiation?
Hebbian learning is the general principle, while long-term potentiation (LTP) is one experimentally observed example of it. LTP is a lasting increase in synaptic strength after certain patterns of activity, first described in rabbit hippocampus by Bliss and Lømo. Because LTP depends on coincident presynaptic and postsynaptic activity, particularly through NMDA receptors, it behaves in a Hebbian way. Not all plasticity is Hebbian, though. Homeostatic scaling, for instance, adjusts synapses based on overall activity, and neuromodulator-driven changes in simple organisms don’t follow the same rule. So LTP is a case of Hebbian plasticity, not a synonym for it.
How does Hebb’s law relate to artificial neural networks?
It’s one of the ancestors. Many early models of learning in artificial networks used Hebb-like rules, in which the weight between two units increases when both are active. Later, more powerful methods such as backpropagation, which adjusts weights to reduce error using information that flows backward through the network, became the standard for deep learning, and they differ from simple Hebbian rules. Researchers still study Hebbian and related biologically inspired rules, partly to understand real brains and partly to build more efficient or brain-like systems. So Hebb’s idea is foundational in spirit, even if modern machine learning mostly uses different algorithms.
Can Hebbian learning explain bad habits and phobias?
Partly. Repeated pairing of a cue with a response can strengthen the circuits linking them, which is consistent with how habits and conditioned fears persist. Exposure therapy, which helps people face feared situations without the feared outcome, works in part by building new learning that competes with the old association. But extinction isn’t simply erasing the original memory; the old association often remains and can return, which is why relapse happens. Hebbian mechanisms are one piece of a bigger picture that includes emotion circuits, reward systems, and context. Treating habits or phobias works best with evidence-based approaches, not neuroscience slogans.
Does practicing more always strengthen the brain connections I want?
Not always. Neurons strengthen whatever they’re actually doing, so practicing mistakes reinforces mistakes. Attention matters, since distracted repetition is often less effective, and spacing practice across days tends to build more durable memory than cramming. Rest and sleep also seem to matter for consolidation. There’s another limit: the brain has stabilizing mechanisms, such as homeostatic plasticity, that keep activity within bounds, so connections don’t strengthen without limit. Quality of practice, meaning accurate, focused, and varied, usually counts for more than raw quantity. If progress stalls despite lots of practice, changing the method often helps more than adding hours.
Who discovered long-term potentiation and why does it matter?
Timothy Bliss and Terje Lømo described it in 1973, working with anesthetized rabbits. They found that brief high-frequency stimulation of the perforant path produced a long-lasting increase in synaptic response in the dentate gyrus of the hippocampus. It mattered because it was the first clear demonstration that synapses can change strength in an enduring, activity-dependent way, as Hebb had hypothesized. Because the hippocampus is essential for forming new declarative memories, LTP became the leading candidate for a cellular basis of memory. Decades of follow-up work have refined and complicated the story, but the original finding remains a landmark of neuroscience.
Bibliography
- Bi, G. Q., & Poo, M. M. (1998). Synaptic modifications in cultured hippocampal neurons: Dependence on spike timing, synaptic strength, and postsynaptic cell type. Journal of Neuroscience, 18(24), 10464-10472.
- Bliss, T. V. P., & Lømo, T. (1973). Long-lasting potentiation of synaptic transmission in the dentate area of the anaesthetized rabbit following stimulation of the perforant path. Journal of Physiology, 232(2), 331-356.
- Hebb, D. O. (1949). The organization of behavior: A neuropsychological theory. Wiley.
- Kandel, E. R. (2001). The molecular biology of memory storage: A dialogue between genes and synapses. Science, 294(5544), 1030-1038.
- Keysers, C., & Perrett, D. I. (2004). Demystifying social cognition: A Hebbian perspective. Trends in Cognitive Sciences, 8(11), 501-507.
- Shatz, C. J. (1992). The developing brain. Scientific American, 267(3), 60-67.
- Turrigiano, G. G., & Nelson, S. B. (2004). Homeostatic plasticity in the developing nervous system. Nature Reviews Neuroscience, 5(2), 97-107.
Use this citation format to reference the article clearly and help readers find the original source.
PsychologyFor. (2026). Hebb’s Law: the Neuropsychological Basis of Learning. PsychologyFor. https://psychologyfor.com/hebbs-law-the-neuropsychological-basis-of-learning/